|
Search Term: " Magnesium Glycinate "
The Ultimate Guide to Cellular Longevity: NAD+, Methylation, and Senolytics   
Date:
September 10, 2026 10:57 AM
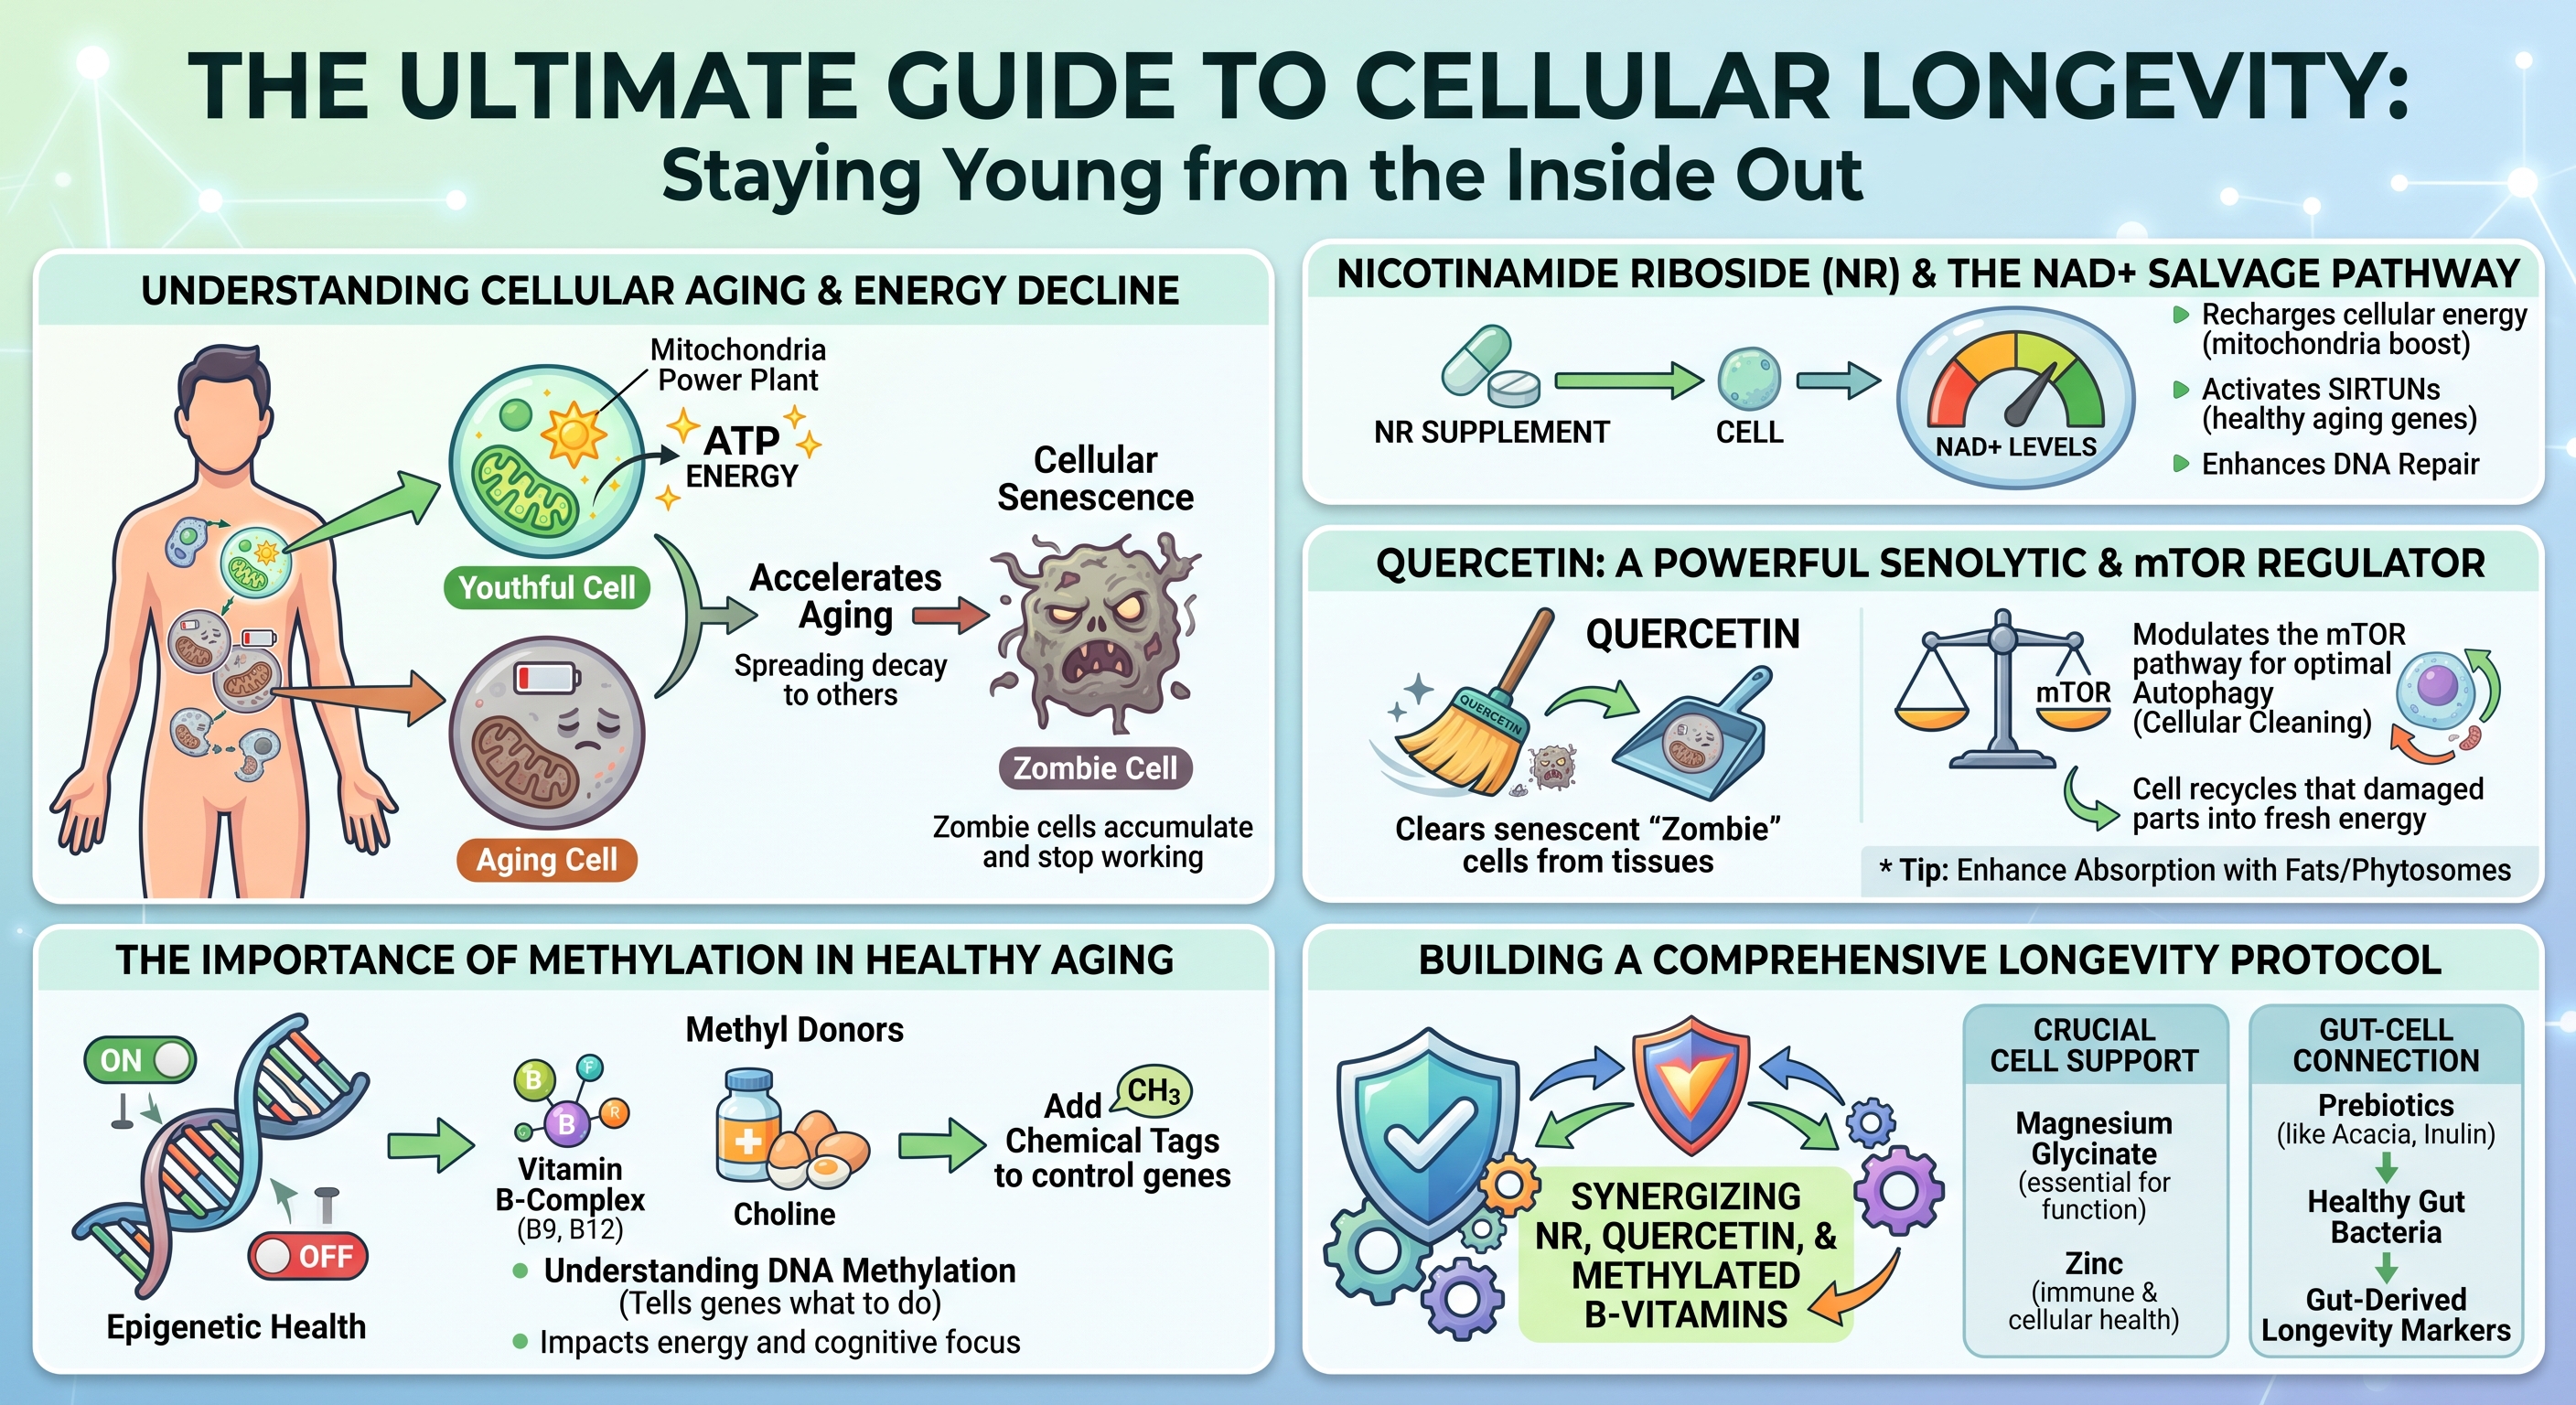
Introduction: Understanding Cellular Aging and Energy DeclineBiological aging represents a progressive decline in cellular maintenance, structural repair, and energy generation. Over decades, tissues experience an attrition of functional reserves, compromised stress resilience, and persistent low-grade systemic inflammation. At the cellular scale, biological degeneration is driven by a failure to generate bioenergetic fuel, repair genetic code, and clear metabolic waste.Cellular aging is characterized by interconnected biological disruptions known as the hallmarks of aging. These encompass genomic instability, epigenetic alterations, mitochondrial decay, loss of proteostasis, and cellular senescence. Rather than operating as isolated occurrences, these phenomena establish a self-reinforcing degenerative cycle: declining cellular power generation impairs enzymatic genetic repair, promoting the accumulation of damaged cells that enter irreversible growth arrest and poison surrounding healthy tissues. Mitigating cellular aging requires examining how microscopic bioenergetic pathways deteriorate and evaluating how targeted nutritional and biochemical interventions can restore cellular homeostasis. The Role of Mitochondria and ATP ProductionEvery biological function - from muscular contraction to continuous DNA replication - depends on adenosine triphosphate (ATP), the primary biochemical energy currency of living systems. Cells produce the vast majority of this energy within mitochondria through oxidative phosphorylation. Within these specialized organelles, metabolic intermediates derived from dietary carbohydrates and lipids donate high-energy electrons to the electron transport chain. The flow of these electrons across protein complexes establishes an electrochemical proton gradient across the inner mitochondrial membrane, driving ATP synthase to manufacture ATP.A youthful cell functions like an efficient municipal power grid, dynamically matching energetic demands with immediate ATP output. However, as biological aging progresses, mitochondrial efficiency declines. The electron transport chain becomes structurally leaky, inadvertently shedding electrons that react with ambient molecular oxygen to produce reactive oxygen species (ROS). While regulated levels of ROS participate in vital intracellular signaling, chronic excess induces widespread oxidative stress. Mitochondria are exceptionally vulnerable to this oxidative burden because they carry their own circular genetic material, known as mitochondrial DNA (mtDNA). Unlike nuclear DNA, mtDNA lacks the protective shielding of histone proteins and possesses rudimentary repair systems. As a result, mtDNA sustains cumulative oxidative damage, encoding increasingly defective electron transport chain proteins. This dynamic generates a bioenergetic deficit: degraded mitochondria synthesize progressively less ATP while emitting greater volumes of damaging free radicals. Deprived of optimal ATP reserves, cells lack the energy necessary to drive vital enzymatic repair cascades, accelerating structural degeneration and functional exhaustion. How Cellular Senescence Accelerates the Aging ProcessWhen healthy cells confront critical physiological damage - such as severe telomere attrition, persistent DNA double-strand breaks, or oxidative stress - they activate protective cell cycle arrest pathways governed primarily by the p53/p21^CIP1 and p16^INK4a/Rb molecular checkpoints. This defensive shutdown, termed cellular senescence, permanently prevents the replication of potentially premalignant or mutated cells.Senescent cells, colloquially known as "zombie cells," enter a state of permanent growth arrest while actively resisting programmed cell death (apoptosis). Over time, these cells accumulate within adipose depots, skeletal muscle, the vascular endothelium, and major organs, largely because immune surveillance and clearance pathways simultaneously lose functional efficiency. The systemic danger of senescent cells stems from their secretome. Rather than remaining biologically inert, senescent cells develop a hyperactive secretory state termed the Senescence-Associated Secretory Phenotype (SASP). The SASP is a destructive mixture of pro-inflammatory cytokines, chemokines, extracellular matrix-degrading matrix metalloproteinases (MMPs), and reactive oxygen species. Through this toxic secretome, even a small burden of senescent cells can impair whole-tissue architecture. SASP factors degrade surrounding structural proteins, induce insulin resistance in neighboring metabolic cells, and biochemically force adjacent healthy cells into secondary senescence. This persistent paracrine signaling fuels chronic, sterile, low-grade systemic inflammation, termed "inflammaging," which accelerates systemic tissue degeneration and elevates susceptibility to degenerative age-related pathologies. Nicotinamide Riboside (NR) and the NAD+ Salvage PathwayThe Biochemistry of NAD+ Depletion Over TimeNicotinamide adenine dinucleotide (NAD+) is an indispensable coenzyme present in every living cell. NAD+ fulfills a dual biological mandate: it serves as a central redox cofactor that shuttles electrons between cellular metabolic reactions, and it functions as an obligatory consumable substrate for regulatory enzymes that preserve cellular viability. In its redox capacity, NAD+ accepts electrons to form NADH during glycolysis, the tricarboxylic acid (TCA) cycle, and fatty acid beta-oxidation, subsequently donating those electrons to Complex I of the respiratory chain to power ATP synthesis.
The primary enzymatic driver of age-related NAD+ destruction is CD38, a membrane-bound glycohydrolase expressed on immune cells that is upregulated in response to chronic SASP exposure. Concurrently, lifelong genotoxic damage causes persistent activation of Poly(ADP-ribose) polymerase 1 (PARP-1), an enzyme that cleaves the glycosidic bonds of NAD+ to assemble branched poly(ADP-ribose) chains at DNA lesion sites. Because PARP-1 consumes NAD+ without directly recycling the molecule, chronic DNA damage depletes intracellular NAD+ pools, impairing bioenergetics and limiting sirtuin activity. How NR Efficiently Boosts Cellular NAD+ LevelsThe mammalian body maintains its NAD+ supply through three distinct biosynthetic routes: the de novo pathway from dietary L-tryptophan, the Preiss-Handler pathway from nicotinic acid (niacin), and the NAD+ Salvage Pathway. The de novo pathway requires substantial energy expenditure, consuming roughly sixty milligrams of dietary tryptophan to yield a single milligram of NAD+. The Preiss-Handler pathway, while effective, can induce cutaneous prostaglandin-mediated flushing at therapeutic intakes. Consequently, the salvage pathway serves as the primary mechanism for maintaining intracellular NAD+ pools.The salvage pathway recycles the breakdown product nicotinamide (NAM), which is released whenever NAD+-consuming enzymes execute their functions. Under normal conditions, cells convert free nicotinamide into nicotinamide mononucleotide (NMN) via the rate-limiting enzyme nicotinamide phosphoribosyltransferase (NAMPT), after which NMN adenylyltransferases (NMNAT1–3) complete the conversion into NAD+. However, NAMPT expression declines with advancing age, chronic inflammation, and metabolic stress, limiting the recycling capacity of the cell. Nicotinamide Riboside (NR) is a naturally occurring pyridine nucleoside that bypasses this enzymatic bottleneck. Upon cellular entry via equilibrative nucleoside transporters, NR is directly phosphorylated into NMN by nicotinamide riboside kinases (NRK1 and NRK2) using a single molecule of ATP. Because the NRK pathway remains intact and robust across the lifespan, NR provides an efficient alternative entry point into the NAD+ salvage cascade. Clinical evaluations in humans confirm the safety, bioavailability, and pharmacokinetics of oral NR supplementation. Randomized, double-blind, placebo-controlled trials reveal that oral NR chloride produces dose-dependent increases in steady-state whole blood NAD+ concentrations. Dosing regimens of 100 mg, 300 mg, and 1,000 mg daily elevate blood NAD+ levels by approximately 22%, 51%, and up to 142%, respectively, within two weeks of administration, maintaining these elevations throughout continuous use. High-resolution metabolomic analyses also demonstrate parallel elevations in nicotinic acid adenine dinucleotide (NAAD), establishing it as a reliable biomarker of active intracellular NAD+ synthesis without hepatic or systemic toxicity. Sirtuin Activation and DNA Repair MechanismsReplenishing intracellular NAD+ supports functions beyond mitochondrial ATP generation. NAD+ functions as an obligatory cofactor for sirtuins (SIRT1 through SIRT7), a family of class III histone and non-histone protein deacetylases that regulate stress resilience, metabolic homeostasis, and cell survival. Sirtuins couple the removal of acetyl groups from target lysine residues to the stoichiometric cleavage of NAD+, producing nicotinamide and O-acetyl-ADP-ribose. In states of NAD+ deficiency, sirtuin enzymes remain inactive regardless of cellular demand.In the nucleus, SIRT1 coordinates defense against cellular decline. When activated by restored NAD+ levels, SIRT1 deacetylates peroxisome proliferator-activated receptor-gamma coactivator 1-alpha (PGC-1a), the master transcriptional coactivator of mitochondrial biogenesis. This deacetylation stimulates mitochondrial replication and assembly, expanding functional respiratory capacity. Concurrently, SIRT1 deacetylates the p65 subunit of nuclear factor-kappa B (NF-kB), suppressing the transcription of pro-inflammatory cytokines. In the mitochondria, SIRT3 utilizes NAD+ to deacetylate metabolic enzymes and superoxide dismutase 2 (SOD2), enhancing the organelle's capacity to neutralize reactive oxygen species. At the same time, cellular NAD+ levels directly regulate genomic integrity through PARP-1. When genotoxic stress or oxidative damage induces single- or double-strand DNA breaks, PARP-1 binds to the damaged termini using its zinc-finger domains. Bound PARP-1 hydrolyzes NAD+ to synthesize extensive, negatively charged poly(ADP-ribose) polymers on itself and adjacent histones. This modification relaxes chromatin architecture and establishes an electrostatic scaffold that recruits base excision repair and homologous recombination complexes. Recent discoveries demonstrate close crosstalk between sirtuins and PARP-1 during DNA repair. PARP-1 recruits SIRT1 to double-strand breaks, where SIRT1 deacetylates the chromatin-remodeling ATPase BRG1 to displace nucleosomes and facilitate homologous recombination. However, because PARP-1 and SIRT1 draw from the same intracellular NAD+ pool, severe NAD+ depletion forces a biological compromise: PARP-1 consumes the scarce remaining cofactor to address DNA damage, leaving sirtuins deactivated. Restoring NAD+ via NR prevents this deficit, enabling concurrent genomic repair and sirtuin-mediated metabolic defense. Quercetin: A Powerful Senolytic and mTOR RegulatorClearing Senescent "Zombie" Cells from TissuesThe accumulation of senescent cells has driven interest in senolytics: molecules that selectively eliminate senescent cells while sparing healthy, non-senescent populations. Senolytic agents exploit a specific vulnerability in senescent cells. Because senescent cells produce cytotoxic, pro-inflammatory SASP factors that would normally induce their own death, they become dependent on upregulated Senescent Cell Anti-Apoptotic Pathways (SCAPs) to survive. The SCAP network involves anti-apoptotic proteins (such as BCL-2 and BCL-xL), the PI3K/Akt kinase cascade, and cyclin-dependent kinase inhibitors.Quercetin is a polyphenolic flavonoid found in capers, red onions, apples, and the flower buds of Sophora japonica. Beyond its classical antioxidant properties, quercetin functions as a senolytic compound that exerts multi-target inhibitory effects across the SCAP network. By inhibiting the upstream PI3K/Akt survival axis and downregulating anti-apoptotic defenses, quercetin disrupts the signaling that protects senescent cells from intrinsic apoptosis. Deprived of these survival signals, senescent cells undergo programmed cell death. Preclinical studies demonstrate that senolytic protocols utilizing quercetin - often combined with the tyrosine kinase inhibitor dasatinib - reduce senescent cell burden across multiple tissues. This targeted clearance lowers circulating SASP factors, attenuates tissue fibrosis, restores endothelial reactivity, and improves functional health span. By removing senescent cells, quercetin mitigates the primary driver of chronic, low-grade inflammaging. Modulating the mTOR Pathway for Optimal AutophagyThe mechanistic Target of Rapamycin (mTOR) is an evolutionarily conserved serine/threonine protein kinase that coordinates cellular metabolism by balancing anabolic growth with catabolic recycling. Operating within two multiprotein complexes - mTORC1 and mTORC2 - the mTOR pathway integrates signals from amino acids, growth factors, and intracellular energy levels. In nutrient-rich environments, mTORC1 promotes protein synthesis, lipogenesis, and cellular growth, while suppressing catabolic breakdown. Conversely, nutrient scarcity downregulates mTORC1, activating autophagy.Autophagy is an intracellular degradation system that packages damaged organelles, misfolded protein aggregates, and biological debris into double-membraned autophagosomes for lysosomal degradation and recycling. A specialized branch of this pathway, mitophagy, selectively targets and clears damaged mitochondria. In modern metabolic conditions characterized by continuous caloric intake, mTORC1 can remain persistently active. This persistent signaling suppresses autophagy, causing damaged organelles and toxic aggregates to accumulate within tissues. Quercetin functions as a natural modulator of mTOR signaling. By inhibiting upstream PI3K/Akt signaling and activating intracellular energy sensors, quercetin attenuates overactive mTORC1, mimicking the metabolic effects of caloric restriction. This down-regulation relieves inhibition on the ULK1 autophagy initiation complex, stimulating both general autophagy and mitophagy. As autophagy proceeds, cells clear protein aggregates and eliminate damaged mitochondria, supporting cellular longevity and proteostasis. Enhancing Absorption: Phytosomes and Dietary FatsDespite the biological activities of quercetin identified in experimental models, its clinical translation has historically been limited by poor oral bioavailability. Raw quercetin aglycone is a crystalline, hydrophobic polyphenol with poor solubility in water and gastrointestinal fluids. When ingested in unformulated powder forms, quercetin molecules aggregate in the gut lumen, resisting dissolution and passive absorption. Consequently, the vast majority of an unformulated dose passes into the colon unabsorbed, where it undergoes microbial degradation without reaching meaningful systemic concentrations.To address these pharmacokinetic limitations, advanced delivery systems such as phytosomes were engineered. A phytosome is a 100% food-grade molecular complex where individual polyphenolic molecules are bound to dietary phospholipids, typically sunflower-derived phosphatidylcholine. Unlike a classical liposome - which encapsulates water-soluble compounds inside an aqueous core enclosed by a lipid bilayer - a phytosome forms an amphiphilic complex at the molecular level. The polar head of the phosphatidylcholine molecule forms hydrogen bonds with the hydroxyl groups of the quercetin molecule, while its lipophilic fatty acid tails extend outward. This structural arrangement shields the polar regions of the flavonoid, creating a lipid-compatible complex that integrates smoothly into the intestinal mucosa.
The Importance of Methylation in Healthy AgingVitamin B-Complex and Choline as Essential Methyl DonorsMethylation is an essential biochemical process occurring billions of times each second across all human tissues. It involves the transfer of a single-carbon unit - a methyl group consisting of one carbon atom bound to three hydrogen atoms - (CH3) - from a donor molecule to diverse recipients, including DNA, RNA, structural proteins, neurotransmitters, and membrane phospholipids. This transfer of one-carbon units is coordinated by the methionine-homocysteine cycle, which sustains genetic stability, detoxification pathways, and cellular repair.At the center of this pathway sits S-adenosylmethionine (SAM), the universal methyl donor in human biology. When a methyltransferase enzyme transfers a methyl group from SAM to an acceptor molecule, SAM is converted into S-adenosylhomocysteine (SAH). SAH functions as a potent competitive inhibitor of intracellular methyltransferases. To maintain functional methylation, SAH is rapidly hydrolyzed into homocysteine, a sulfur-containing amino acid that must be remethylated or cleared through transsulfuration. Homocysteine clearance proceeds through two distinct remethylation pathways. The primary route operates across most tissues via the enzyme methionine synthase, which requires vitamin B12 in its active methylcobalamin form. Methionine synthase transfers a methyl group from 5-methyltetrahydrofolate (5-MTHF, the active form of folate) to homocysteine, regenerating methionine. The ongoing production of 5-MTHF depends on the enzyme methylenetetrahydrofolate reductase (MTHFR), which utilizes riboflavin (vitamin B2) as a cofactor. Alternatively, excess homocysteine can be routed into the transsulfuration pathway by vitamin B6 (as pyridoxal-5'-phosphate) to synthesize cystathionine, cysteine, and ultimately the antioxidant glutathione. A secondary remethylation pathway, active predominantly in hepatic and renal tissues, bypasses folate entirely. In this route, dietary choline is oxidized to betaine (trimethylglycine or TMG). The enzyme betaine-homocysteine S-methyltransferase (BHMT) then transfers a methyl group from betaine directly to homocysteine, yielding methionine and dimethylglycine. When dietary intake of active B-vitamins or choline is insufficient, or when genetic variations like MTHFR polymorphisms reduce pathway flux, the methylation cycle slows. Homocysteine accumulates in circulation, promoting vascular and neurological inflammation, while SAM reserves decline, restricting cellular methylation capacity. Understanding DNA Methylation and Epigenetic HealthEvery somatic cell in an organism carries an identical genetic code. Cellular differentiation and tissue-specific functions are governed by the epigenome: a regulatory layer of chemical modifications that dictates gene expression without altering underlying DNA sequences. DNA methylation represents the primary and most stable epigenetic modification. In this process, DNA methyltransferase (DNMT) enzymes utilize methyl groups donated by SAM to add a methyl tag to cytosine bases adjacent to guanine residues, forming 5-methylcytosine within CpG dinucleotide sites.Under physiological conditions, DNA methylation maintains genomic stability and coordinates transcription. Methylation of promoter regions condenses chromatin, repressing transposable elements and silencing genes inappropriate for a given cell type. Conversely, hypomethylated promoters maintain an open chromatin state, allowing transcription factors to bind and initiate gene expression. During biological aging, this epigenetic landscape undergoes progressive dysregulation, a phenomenon termed "epigenetic drift". Aging cells experience global hypomethylation alongside focal hypermethylation of specific gene promoters. Global loss of methyl tags destabilizes the genome, activating retrotransposons and pro-inflammatory pathways. Simultaneously, hypermethylation at targeted promoter sites silences critical tumor suppressor genes and DNA repair complexes. This systematic change in DNA methylation patterns is consistent across populations, allowing researchers to develop molecular "epigenetic clocks". Algorithms such as the Horvath clock, PhenoAge, and GrimAge quantify biological age by profiling the methylation status of specific CpG sites across the genome. These clocks assess whether individuals are aging faster or slower than their chronological years. Ensuring a steady supply of methyl donors and preventing unnecessary SAM depletion supports DNMT activity, maintaining epigenetic patterns and genomic stability. How the Methylation Cycle Impacts Energy and Cognitive FocusBeyond long-term epigenetic regulation, the methylation cycle directly modulates immediate biochemical processes that govern daily energy, neurotransmission, and cognitive focus. Compromised methylation capacity frequently manifests as cognitive slowing, executive fatigue, and reduced physical stamina.A major consumer of methyl reserves is the endogenous synthesis of creatine. Approximately 40% of all SAM-derived methyl groups in the human body are utilized by guanidinoacetate N-methyltransferase (GAMT) in the liver to synthesize creatine. Creatine then translocates to the brain and skeletal muscle, where it is phosphorylated into phosphocreatine. Phosphocreatine functions as a rapid energy buffer, donating a high-energy phosphate group to regenerate ADP into ATP in milliseconds during demanding physical or cognitive tasks. When methyl donor availability falls, endogenous creatine synthesis drops, depleting phosphocreatine reserves and increasing susceptibility to neuromuscular and cognitive fatigue. Methylation is equally central to central nervous system architecture. SAM provides methyl groups to convert phosphatidylethanolamine into phosphatidylcholine, the predominant phospholipid comprising neuronal cell membranes and the myelin sheaths that insulate axons. Intact myelin preserves rapid action potential conduction throughout the nervous system. Furthermore, free choline derived from this pathway is the direct precursor to acetylcholine, the neurotransmitter required for attention, working memory, and learning. The methylation cycle also governs monoamine neurotransmitter metabolism. SAM is required for the synthesis of adrenaline (epinephrine) from noradrenaline, while catechol-O-methyltransferase (COMT) relies on SAM to degrade dopamine and norepinephrine within the prefrontal cortex. Sluggish methylation disrupts this balance, contributing to cognitive fatigue, mood variability, and impaired mental performance. Building a Comprehensive Longevity ProtocolSynergizing NR, Quercetin, and Methylated B-VitaminsLongevity supplementation often falters when single molecules are administered in isolation, ignoring interconnected metabolic pathways. Designing an effective cellular longevity protocol requires combining complementary mechanisms that reinforce one another while preventing secondary metabolic deficits. The combination of Nicotinamide Riboside, Quercetin Phytosome, and Methylated B-Vitamins illustrates this multi-target synergy.This synergy is grounded in the direct biochemical intersection between the NAD+ salvage pathway and the methylation cycle. When high-dose NR is supplemented to boost systemic NAD+, sirtuins and PARP enzymes consume the newly synthesized cofactor, generating substantial quantities of free nicotinamide (NAM). This intracellular nicotinamide faces two primary metabolic fates: it can be recycled back into NAD+ through the NAMPT-dependent salvage loop, or it can be cleared via methylation. When the influx of nicotinamide exceeds salvage recycling capacity, the excess is cleared to avoid feedback inhibition of sirtuin enzymes. To accomplish this, the enzyme nicotinamide N-methyltransferase (NNMT) transfers a methyl group from SAM directly onto nicotinamide, forming 1-methylnicotinamide (1-MNA/MNAM), which is subsequently excreted in urine. Prolonged, high-dose precursor administration without nutritional methyl support can elevate NNMT flux, depleting intracellular SAM reserves. As methyl groups are consumed clearing nicotinamide, the cellular SAM-to-SAH ratio falls, which can elevate circulating homocysteine and reduce methyl availability for DNA methylation and neurotransmitter synthesis. Co-administering a fully methylated B-complex alongside choline or betaine addresses this potential bottleneck. Providing active methyl donors (such as 5-MTHF, methylcobalamin, and betaine) maintains the one-carbon donor pool. Even during increased NNMT activity, SAM pools remain stable, protecting DNA methylation fidelity and maintaining homocysteine within safe parameters. Quercetin reinforces this protocol through complementary mechanisms. By clearing senescent cells and reducing SASP-mediated inflammation, quercetin downregulates CD38, the primary enzyme responsible for age-related NAD+ degradation. Suppressing CD38 prevents unnecessary breakdown of newly synthesized NAD+, enhancing the efficiency of NR supplementation. Furthermore, while NR provides the NAD+ necessary to activate SIRT1-driven mitochondrial biogenesis, quercetin concurrently modulates mTORC1 to stimulate autophagy. This coordinated action ensures that newly generated mitochondria operate in an environment cleared of proteotoxic cellular debris. The Crucial Role of Magnesium Glycinate and Zinc in Cellular FunctionLongevity protocols require essential mineral cofactors to function efficiently. Without adequate divalent minerals acting as enzymatic cofactors and structural stabilizers, metabolic longevity pathways cannot operate at full capacity. Among these, magnesium and zinc are required for cellular repair, genomic stability, and energy production.Magnesium serves as an obligatory cofactor in over 300 enzymatic reactions, primarily through its interaction with ATP. In biological systems, ATP exists predominantly as a chelate with a divalent magnesium ion, forming biologically active Mg2+ -ATP. Every enzymatic reaction that synthesizes, transfers, or consumes cellular energy - including the enzymes of the NAD+ salvage pathway (NRK and NMNAT) and DNA polymerases - strictly requires Mg2+ -ATP as its substrate. Magnesium deficiency impairs these phosphorylation reactions, reducing the cellular utilization of NAD+ precursors. Additionally, magnesium is an essential cofactor for the enzymes that activate dietary B-vitamins into their active forms. Supplying magnesium as Magnesium Glycinate provides high gastrointestinal bioavailability, minimal laxative effect, and yields glycine to support inhibitory neurotransmission and restful sleep. Zinc serves as a vital structural component for more than 3,000 human transcription factors and enzymatic proteins. Its most prominent structural role in longevity occurs within zinc-finger motifs. These are specialized protein conformations stabilized by a zinc ion coordinated to cysteine and histidine residues. The DNA damage sensor PARP-1 utilizes three zinc-finger domains to identify, track, and physically bind to single- and double-strand DNA breaks. Without adequate intracellular zinc, PARP-1 cannot properly assemble or dock onto damaged chromosomes, impairing DNA repair and increasing genomic instability. Zinc is also an obligatory structural component of copper/zinc superoxide dismutase (Cu/Zn-SOD or SOD1), the primary cytosolic antioxidant enzyme that dismutates superoxide radicals into hydrogen peroxide, protecting mitochondrial membranes and nuclear DNA from premature senescence. Integrating Prebiotics (like Acacia and Inulin) for Gut-Derived Longevity MarkersA comprehensive cellular longevity framework must extend beyond somatic tissues to encompass the gut microbiome. The intestinal microbiome functions as a central regulator of systemic inflammatory tone, immune development, and metabolic signaling. Age-associated dysbiosis - characterized by the loss of beneficial commensals and an overgrowth of pathobionts - frequently leads to breakdown of the intestinal barrier.The gut epithelium consists of a single-cell monolayer sealed by tight junction proteins, including zonula occludens-1 (ZO-1), occludin, and claudins. When this physical barrier is disrupted by poor dietary fiber intake or dysbiosis, gut permeability increases. This allows lipopolysaccharide (LPS), a component of the outer membrane of Gram-negative bacteria, to enter the portal and systemic circulation. The resulting "metabolic endotoxemia" activates Toll-like receptor 4 (TLR4) on immune cells, inducing NF-kB and systemic pro-inflammatory cytokine production. This persistent gut-derived inflammation exacerbates the SASP, accelerates tissue senescence, upregulates CD38, and drains systemic NAD+ reserves.
These short-chain fatty acids, particularly butyrate, exert direct protective effects on systemic longevity. Butyrate provides the primary metabolic fuel for colonic epithelial cells, supplying more than 70% of their baseline energy needs and supporting mitochondrial function within colonocytes. Furthermore, SCFAs upregulate the expression of epithelial tight junction proteins (ZO-1, occludin, and claudin-1), restoring intestinal barrier integrity and preventing the translocation of inflammatory LPS into systemic circulation. Systemically absorbed butyrate also functions as an endogenous histone deacetylase (HDAC) inhibitor, suppressing pro-inflammatory gene expression and supporting regulatory T cell (T_reg) development. Reducing metabolic endotoxemia dampens systemic inflammation, protecting vascular function and preventing premature NAD+ depletion. Conclusion: The Integrated Cellular Longevity MatrixCellular longevity is achieved not by addressing isolated biomarkers in isolation, but by systematically supporting interconnected biological pathways. As bioenergetic capacity declines, cellular senescence accelerates, epigenetic patterns degrade, and gut barrier integrity weakens. A comprehensive approach addresses these biological vulnerabilities simultaneously.
Quercetin Phytosome clears senescent cells and modulates mTORC1, stimulating autophagy while dampening the inflammatory SASP cascade that accelerates CD38-mediated NAD+ destruction. Methylated B-vitamins, active folate, and choline replenish SAM reserves, balancing the methyl requirements of NNMT-mediated nicotinamide clearance, preserving epigenetic DNA methylation, and maintaining neurotransmitter production. Magnesium Glycinate and zinc provide the structural and catalytic foundation required for ATP utilization, B-vitamin activation, and PARP-1 zinc-finger DNA repair docking. Finally, prebiotic fibers generate short-chain fatty acids like butyrate, reinforcing the intestinal barrier and preventing metabolic endotoxemia from fueling systemic inflammation. By coordinating energy replenishment, cellular waste clearance, epigenetic maintenance, and the suppression of systemic inflammation, this unified approach directly addresses the underlying drivers of cellular aging to support long-term physiological vitality.
--
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=6650) The Silent Deficiency: Why 60% of Americans Are Running on Empty (and How to Fix It) 
Date:
April 15, 2026 02:04 PM
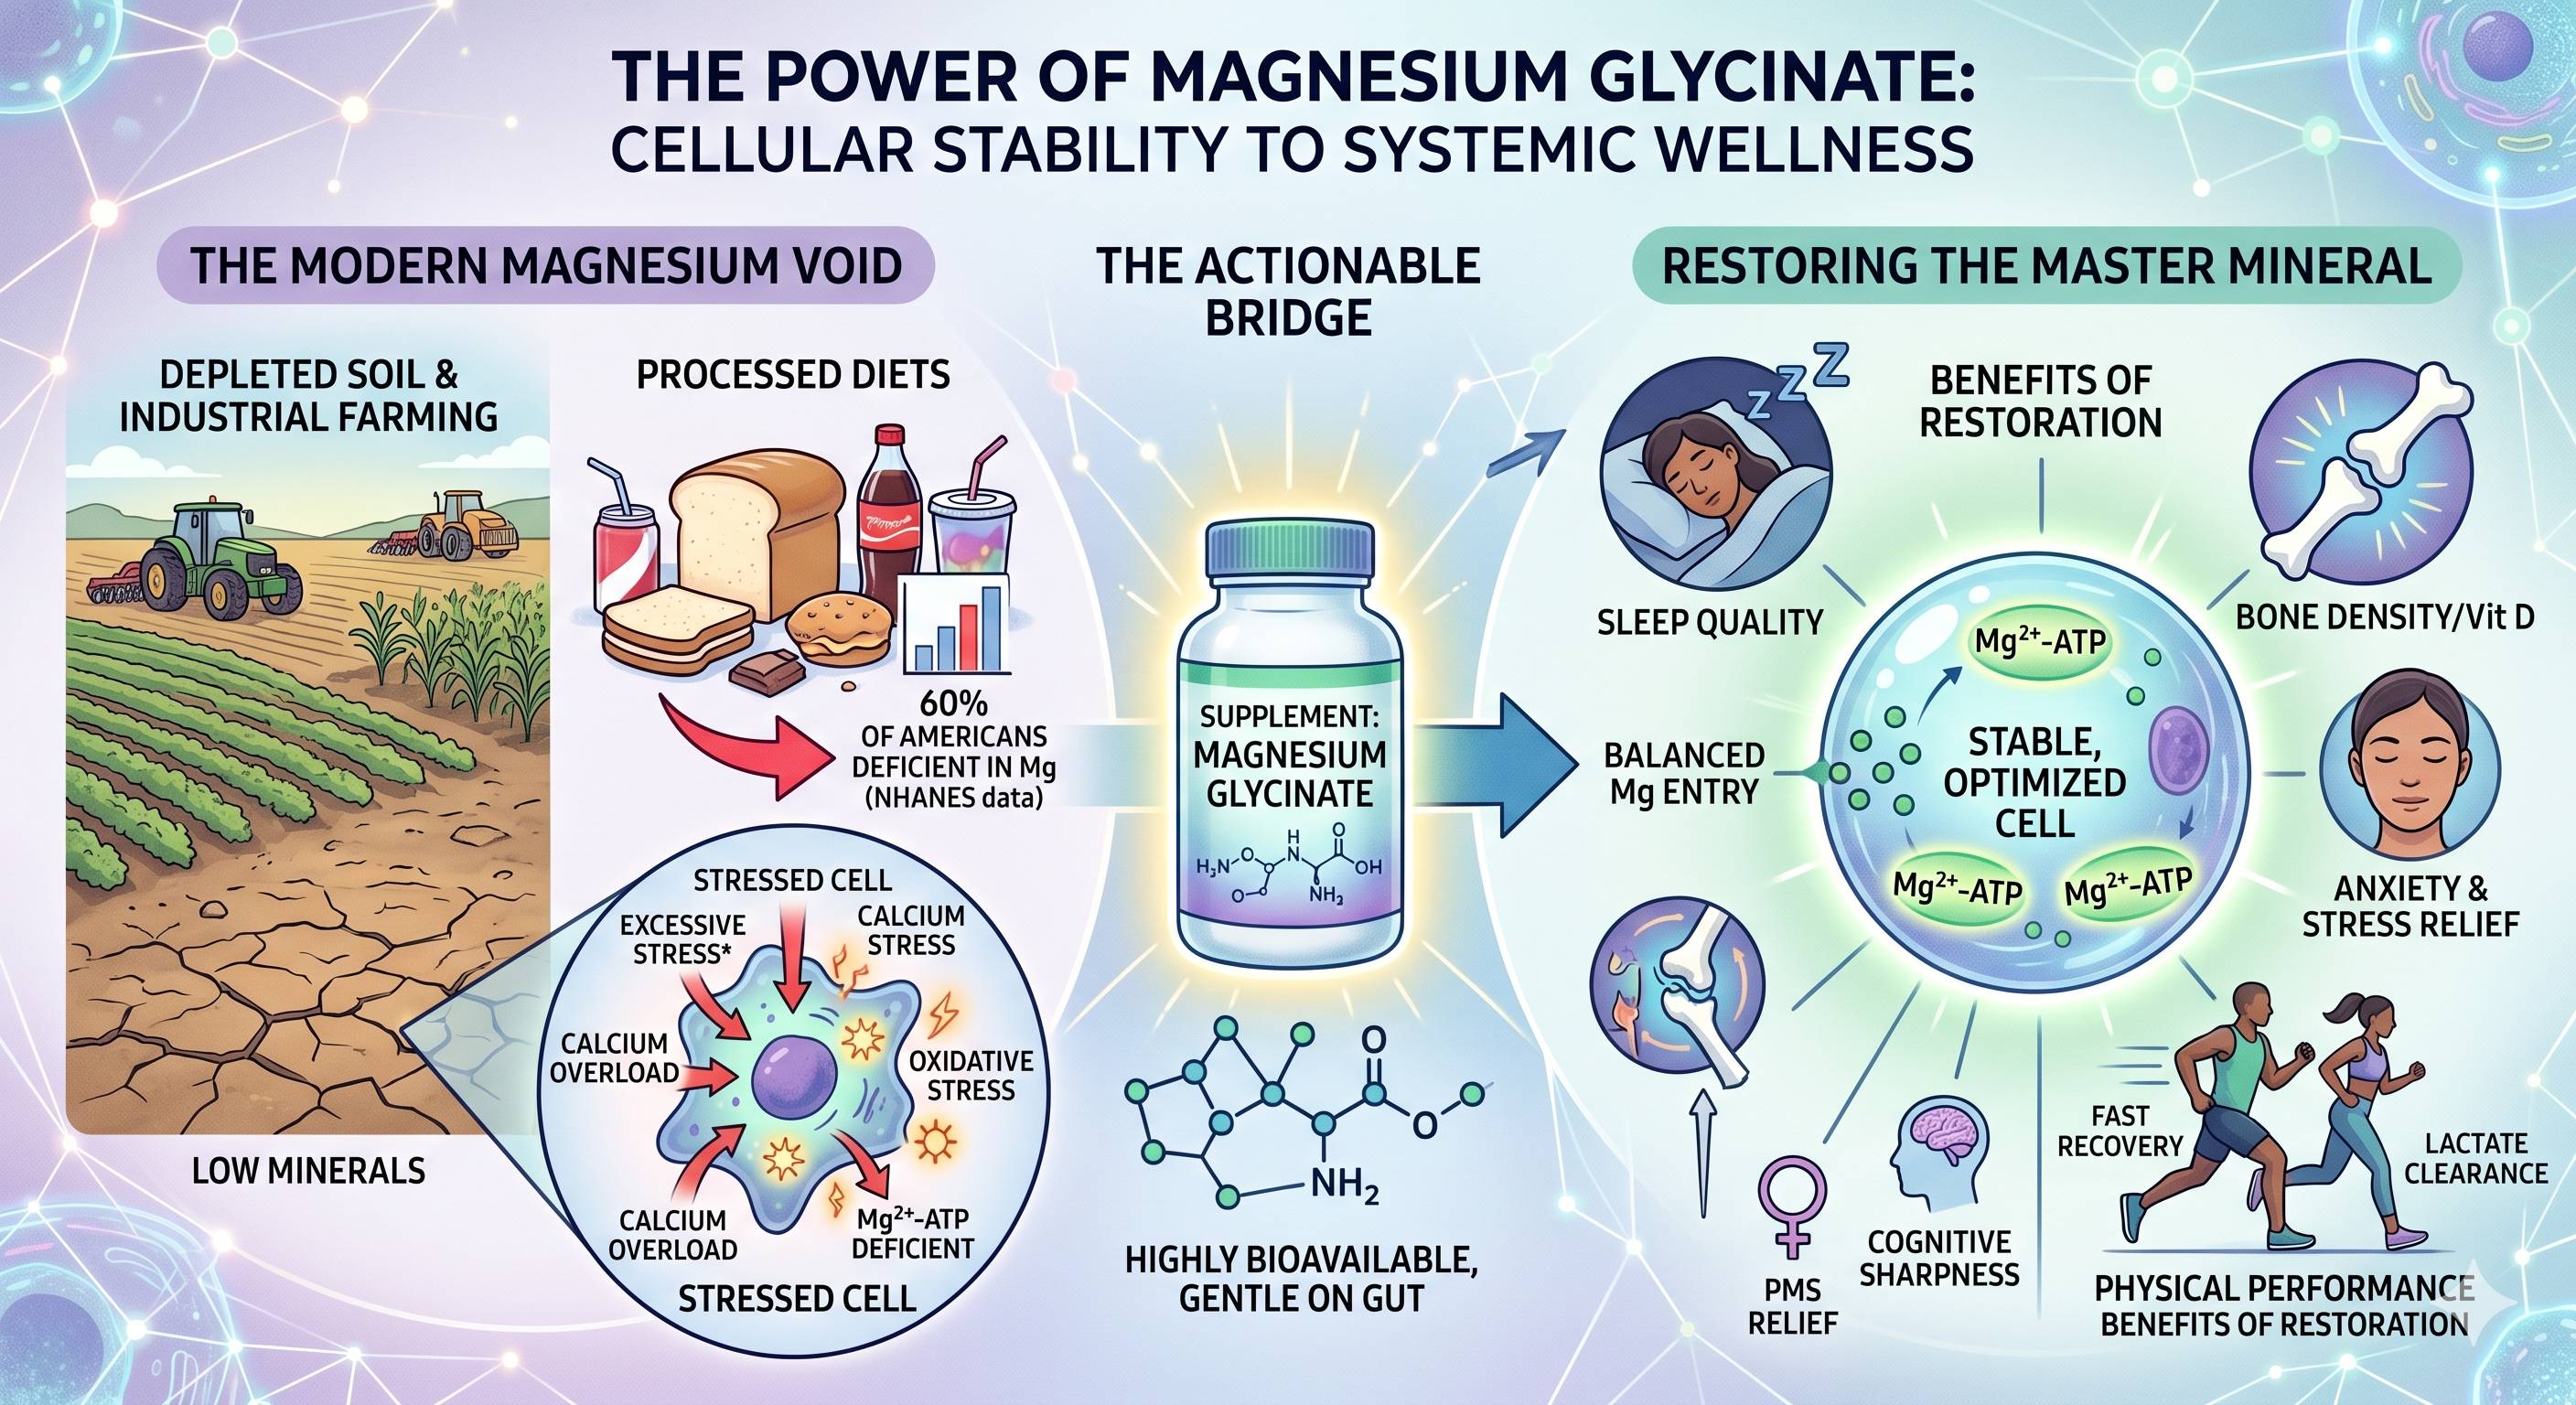
Cellular Stability: The Body's "Brake" SystemAt a cellular level, magnesium is essential for maintaining the structural integrity of membranes. It acts as a natural calcium channel blocker.When you are under stress, your cells can become flooded with calcium, which "excites" the cell. Magnesium sits at the "gate," ensuring that only the necessary amount of calcium enters. Without enough magnesium, cells become hyper-excitable, leading to oxidative stress, inflammation, and even cell death. Furthermore, magnesium is a required co-factor for the production and stability of ATP (adenosine triphosphate), the primary energy currency of the cell. In fact, ATP is usually found in the body as a complex called Mg^2+-ATP. Why Our Modern World is Magnesium-PoorEven if you eat your greens, you might still be coming up short. Here is why:1. Depleted SoilIndustrial farming practices - specifically monocropping and the heavy use of NPK (nitrogen, phosphorus, potassium) fertilizers - have stripped the soil of trace minerals. NPK fertilizers help plants grow tall and look "healthy," but they don't replenish the magnesium that used to be naturally present in the earth. If it’s not in the soil, it’s not in the plant.2. Food ProcessingThe "Standard American Diet" is a magnesium desert. Processing grains to make white flour removes the germ and bran, where the vast majority of magnesium resides. Similarly, refining sugar and oils strips away minerals, leaving us with "empty" calories that actually require more magnesium to metabolize.The "Invisible" DeficiencyHow many Americans are deficient? The statistics are startling. Most nutritional surveys, including NHANES data, suggest that roughly 50% to 60% of the American public do not meet the Recommended Dietary Allowance (RDA) for magnesium.However, many functional medicine experts argue this number is actually higher because the RDA is designed to prevent acute deficiency, not to optimize health. Furthermore, magnesium is stored in bones and soft tissue, not the blood, meaning standard "Serum Magnesium" blood tests often miss a deficiency until it is dangerously low. The Gold Standard: Magnesium GlycinateIf you are looking to supplement, Magnesium Glycinate is widely considered the superior choice.Unlike Magnesium Oxide (which has poor absorption) or Magnesium Citrate (which can have a laxative effect), Magnesium Glycinate is chelated with the amino acid glycine. This makes it:
Benefits of Restoring Magnesium LevelsOnce your cellular "bank account" for magnesium is topped up, the changes can feel transformative:
Further benefits:While we’ve touched on the "big hitters" like sleep and stress, magnesium is involved in over 300 biochemical reactions. When you restore your levels, you’re essentially "re-tuning" several internal systems that may have been glitchy for years.Here are the additional benefits you might notice once your magnesium "tank" is full: Structural & Bone StrengthWe often give calcium all the credit for strong bones, but magnesium is the "manager" that tells calcium where to go.
Hormonal Harmony & PMS ReliefFor women, magnesium is a game-changer for the monthly cycle.
Physical Performance & RecoveryIf you exercise, magnesium is your best friend for "bouncing back."
Cognitive Sharpness & NeuroprotectionRestoring magnesium doesn't just calm the brain; it clears it.
Respiratory EaseMagnesium is a natural bronchodilator.
DNA Integrity & Anti-AgingOn the most microscopic level, magnesium is a "repairman."
Magnesium acts as the body's essential "biological coolant," stabilizing cellular integrity by regulating calcium influx and powering nearly every metabolic process as a co-factor for Mg^2+-ATP. Despite its critical role, more than half of the American population remains chronically deficient, a silent crisis fueled by mineral-depleted industrial soil and the stripping of nutrients during food processing. Transitioning to a high-quality supplement like Magnesium Glycinate offers a superior path to replenishment because its chelated form is both highly bioavailable and gentle on the digestive system. Once levels are restored, the systemic "re-tuning" manifests as a profound shift in well-being, ranging from enhanced sleep quality and stress resilience to improved bone density, hormonal balance, and DNA repair, effectively moving the body from a state of hyper-excitable stress to one of optimized physiological stability.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=6637) Magnesium Glycinate: An In-Depth Guide
Date:
November 04, 2023 10:53 AM
Magnesium Glycinate: An In-Depth GuideMagnesium is an essential mineral for the body, playing a crucial role in the regulation of blood pressure and numerous other bodily functions. The shortcoming of this nutrient can be addressed through the consumption of Magnesium Glycinate, a supplement also known as magnesium diglycinate and magnesium bisglycinate. Key Roles of Magnesium
This article delves into the details of Magnesium Glycinate, looking at its benefits, potential side effects, the recommended dosage, and more. Benefits of Magnesium GlycinateThe human body needs a significant amount of magnesium for optimal function. Although the best way to obtain nutrients is in their natural form, supplements like Magnesium Glycinate are available to enhance magnesium intake in individuals with low levels. Benefits of this supplement include:
Precautionary Measures
Conditions that may Benefit from Magnesium Glycinate
Sources of Magnesium Glycinate Nutritional sources rich in magnesium include legumes, nuts, seeds, whole grains, spinach, fortified breakfast cereals, yogurt, milk, and other dairy products. Recommended Dosage The amount of Magnesium Glycinate to be taken can vary. It is advised to consult a doctor before starting a Magnesium Glycinate regimen. Potential Side Effects Magnesium Glycinate, like other dietary supplements, can cause side effects such as nausea, abdominal cramps, and diarrhea when taken in large or frequent doses. However, a study from 2013 indicated that Magnesium Glycinate is less likely to induce diarrhea compared to other magnesium supplements. Extreme doses could lead to magnesium toxicity, resulting in more severe side effects. Easy Ways to Consume More Magnesium One effective method of increasing magnesium intake is by incorporating dietary supplements into your daily regime. For instance, Solaray Magnesium Glycinate is a popular supplement that is widely recognized for its efficacy. It is an easily digestible form of magnesium that is gentle on the stomach and less likely to induce diarrhea. Solaray's supplement provides an accessible option for those looking to supplement their diet with magnesium, especially for individuals who might struggle to meet their nutritional requirements through diet alone. Conclusion Magnesium Glycinate can be a beneficial supplement for individuals with magnesium deficiency. However, caution must be exercised in its consumption, with potential side effects and individual health conditions taken into account. As always, it is best to seek medical advice before starting a new supplement regimen.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=6587) What Are The Health Benefits Of Magnesium Glycinate?
Date:
March 12, 2013 11:58 AM
Magnesium Glycinate is derived from the attachment of magnesium to glycine. The health benefits of Magnesium Glycinate are many. Naturally, the body needs magnesium to function properly. If the magnesium levels in our blood are less than normal, it is necessary to take Magnesium Glycinate supplement. When the amount of magnesium in the human body is very low, it may lead to various ailments. Likewise, excessive intake of this nutrient may lead to fatigue, vomiting, nausea, diarrhea etc. Let us consider some of the health benefits of this supplement: Prevent High blood pressure Medical Experts believe that consuming a large amount of this supplement can help prevent or reduce the effect of high blood pressure. Individuals who are already suffering from high blood pressure can take this supplement to reduce hypertension. Increase Levels of HDL HDL stands for good cholesterol. This supplement can also help reduce levels of bad cholesterol and increase levels of good cholesterol. Improve Sleep Quality People who have low levels of magnesium may find it difficult to sleep. If you are yet to achieve a more restful sleep, perhaps you can take this supplement. Those who are struggling with restless leg syndrome may also find this supplement helpful. Mood enhancer Magnesium Glycinate supplement can help balance your mood swings. According to the author of "Healing Depression Naturally" Lewis Harrison, magnesium has the ability to regulate neurotransmitter receptor sites. Harrison emphasizes on the use of Magnesium Glycinate as a good treatment for depression. He stated that Magnesium Glycinate helps to remove mercury from the body, which can lead to emotional stability. However, this claim is based on anecdotal evidence and not clinical studies. Notwithstanding, some persons have achieved success using this supplement to treat depression. Therefore, if you are struggling with fatigue, sleeplessness, depression, high blood pressure and high bad cholesterol levels, then this supplement is for you.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=2829) Benefits of Total Daily Formula
Date:
October 13, 2005 04:45 PM
Benefits of Total Daily Formula All fruits and vegetables contain carotenes, the plant pigments responsible for the rich variety of colors we enjoy in the natural world. Beta carotene is the most familiar member of the carotene family. But beta carotene never exists by itself; it is always found with other carotenes in foods. We need more than just beta carotene alone. Carotenes are powerful antioxidants, which means they help reduce the body's free radical burden. Research suggests that carotenes work as a team to keep us healthy.5 Total Daily Formula provides beta carotene, alpha carotene, lutein, lycopene, zeaxanthin and cryptoxanthin from natural sources such as algal extracts, carrot oil, marigold and tomatoes (Caromix®). Total Daily Formula uses only corn-free vitamin C (ascorbic acid). The full daily intake of 6 tablets provides an exceptionally generous 800 mg of vitamin C. Total Daily Formula supplies ample amounts of all essential B vitamins. Vitamin B3 is given as niacin plus an extra helping of niacinamide, the non-flush form of this important vitamin. The body uses pantothenic acid (vitamin B5) to deal with stress, so the formula provides 150 mg, which is 15 times the RDA. Vitamin B6 is another B vitamin people may run short of, so 60 mg -- 30 times the RDA -- is supplied. The formula contains 800 mcg of folic acid, the vitamin now recognized by the FDA as essential for prevention of neural tube defects in unborn babies. Folic acid also helps prevent accumulation in the body of homocysteine, a metabolite of the amino acid methionine.6 A high blood homocysteine level is now considered to be a risk factor for heart disease.7 Flavonoids, also known as "bioflavonoids." are plant pigments widely distributed throughout the plant kingdom.8 Previously known as "Vitamin P," because they help reduce capillary permeability (leakiness) flavonoids are now regarded as "semi-essential" non-vitamin nutrients that benefit health in a variety of ways.9 In addition to maintaining the structure of blood vessels, flavonoids function as versatile antioxidants. Flavonoids protect vitamin C from destruction by free-radicals, helping to preserve the body's vitamin C supply.10 Total Daily Formula provides 100 mg of pure flavonoids from 112 mg of citrus extract. Three superior sources of Calcium Total Daily Formula contains three of the best absorbed and most effective forms of calcium available. MCHC (microcrystalline hydroxyapatite concentrate) is a naturally-derived compound composed of calcium, plus all the minerals and organic factors in living bone tissue. MCHC has been clinically shown to benefit bone health.11 Calcium citrate malate is a very well-absorbed form of supplemental calcium shown in recent research to be helpful for postmenopausal women.12,13 Calcium glycinate is chelated with the amino acid glycine, one of the most efficient mineral carriers for effective absorption.14,15 Magnesium is essential for strong bones and healthy hearts. This versatile mineral also regulates nerve function, keeps muscles relaxed and coordinates activity of over 300 enzymes in the body.16 Total Daily Formula contains 100 percent Magnesium Glycinate for exceptional absorption and gentleness on the intestinal tract.17 Magnesium Glycinate has been clinically tested on people with severe malabsorption with excellent results.18 Total Daily Formula provides - in addition to zinc, chromium, selenium and iodine - vanadium and molybdenum. Vanadium helps maintain normal blood sugar.19 Molybdenum works as a co-factor for enzymes that help detoxify and eliminate foreign substances from the body.20 Bioperine® for Enhanced Absorption Bioperine® is a natural extract derived from black pepper that enhances nutrient absorption. Preliminary trials on humans have shown significant increases in the absorption of nutrients consumed along with Bioperine®. 21 Betaine HCL - supplies HCL (hydrochloric acid) to assist digestion. All natural tablet coating made of vegetable concentrate and beta carotene.
Scientific References 2. Morgan, K.J. et. al. Magnesium and calcium dietary intakes of the U.S. population. Journal of the American College of Nutrition. 1985;4:195-206. 3. Lakschmanan, F.L., Rao, R.B., Kim, W.W., Kelsay, J.L. Magnesium intakes, balances and blood levels of adults consuming self-selected diets. American Journal of Clinical Nutrition 1984;40:1380-89. 4. Mertz, W. The Essential Trace Elements. Fed. Proc. 1970;29:1482. 5. Perry, G. Byers, T. Dietary carotenes, vitamin C and vitamin E as protective antioxidants in human cancers. Annu. Rev. Nutr. 1992;12:139-59. 6. Landgren, F., et. al. Plasma homocysteine in acute myocardial infarction: Homocysteine-lowering effect of folic acid. J Int Med 1995;237:381-88. 7. Clarke, R., et. al. Hyperhomocysteinemia: an independent risk factor for vascular disease. New Eng J Med 1991;324:1149-55. 8. Havsteen, B. Flavonoids, a class of natural compounds of high pharmacological potency. Biochemical Pharmacology 32(7):1141-48. 9. Middleton, E. The flavonoids. TIPS 1984; 5:335-38. 10. Roger, C.R. The nutritional incidence of flavonoids: some physiological and metabolic considerations. Experientia 44(9):725-804. 11. Dixon, A. St. J. Non-hormonal treatment of osteoporosis. British Medical Journal 1983;286(6370):999-1000. 12. Smith, K.T. et. al. Calcium Absorption from a new calcium delivery system (CCM). Calcif Tissue Int 1987;41:351-352. 13. Dawson-Hughes, B. et. al. A controlled trial of the effect of calcium supplementation on bone density in postmenopausal women. New England Journal of Medicine 1990 Sep 27;323(13):878-883. 14. Albion Research Notes Vol. 4, No. 1, ©Albion Laboratories Jan,1995. 15. Ashmead, H.D. Intestinal Absorption of Metal Ions and Chelate, Springfield: Charles C Thomas, ©1985. 16. Wester, P.O., Dyckner, T. The importance of the magnesium ion. Magnesium deficiency-symptomatology and occurrence. Acta Med Scand 1992; (Suppl) 661:3-4. 17. Albion Research Notes Vol. 3, No. 1, ©Albion Laboratories, Feb 1994. 18. Schutte, S., et. al. Bioavailability of Mg diglycinate vs MgO in patients with ileal resections. Abstract 115, AJCN 1992;56(4). 19. Cohen, N. et. al. Oral vanadyl sulfate improves hepatic and peripheral insulin sensitivity in patients with non-insulin-dependent diabetes mellitus. J. Clin Invest 1995; 95:2501-09. 20. Sardesi, V.M. Molybdenum: An essential trace mineral element. Nutr Clin Pract 1993; 8:277-81. 21. Bioperine® - Nature's Bioavailability Enhancing Thermo-nutrient. Executive Summary' 1996; Sabinsa Corporation, Piscataway, N.J.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=839)
Date:
October 06, 2005 10:08 PM
Magnesium is a dietary mineral with a wide array of biological activities in the body. Magnesium participates in numerous life-essential processes that occur both inside and outside cells. Magnesium deficiency impacts normal physiologic function on many levels. Adequate magnesium is a fundamental requirement for optimum function of the cardiovascular system, the nervous system and skeletal muscle, as well as the uterus and GI tract. Magnesium deficiency can affect health of the heart, bones and blood vessels and alter blood sugar balance [1]. Magnesium–Important for Everyone, Deficient in Many The average person living in a modern country today very likely consumes less than the optimum amount of magnesium [2]. An abundance of data collected over the last two decades shows a consistent pattern of low magnesium intake in the U.S. This pattern cuts a wide swath across various age-sex groups. The USDA’s Nationwide Food Consumption Survey found that a majority of Americans consumed less than the recommended daily magnesium intake [3]. Twelve age-sex groups were studied and this low magnesium intake was true for all groups except 0 to 5 year olds. An analysis of the nutrient content of the diets of 7,810 individuals age four and above included magnesium among several nutrients where the amounts supplied by the average diet "were not sufficient to meet recommended standards" [4]. The FDA’s Total Diet study examined the intakes of eleven minerals, including magnesium, among eight age-sex groups. Data was collected four times yearly from 1982 to 1984. Levels of magnesium, calcium, iron, zinc and copper were low for most age-sex groups [5]. Surveys conducted in Europe and in other parts of North America paint a similar picture. Loss of magnesium during food processing is one explanation for this global lack of adequate dietary magnesium [6]. In particular, the elderly may be susceptible to magnesium deficiency for a variety of reasons, including inadequate magnesium intake, poor absorption due to impaired gastrointestinal function and use of drugs such as diuretics that deplete magnesium from the body [7]. It has recently been theorized that magnesium deficiency may contribute to accelerated aging, through effects on the cardiovascular and nervous systems, as well as muscles and the kidneys [8]. Women who take both synthetic estrogen and calcium supplements may be at risk for low blood levels of magnesium [9]. Estrogen promotes the transfer of magnesium from blood to soft–tissues. Low blood magnesium may result if the ratio of calcium to magnesium intake exceeds 4 to 1. Magnesium supplementation is thus advisable for women taking estrogen and calcium. Young adults are not immune to magnesium deficiency. The University of California’s Bogalusa Heart Study collected nutritional data from a cross-sectional sample of 504 young adults between age 19 and 28 [10]. The reported intake of magnesium, along with several other minerals and vitamins, was below the RDA. Glycine is a highly effective mineral chelator. This is because it is a low-molecular-weight amino acid, hence is easily transported across the intestinal membrane. A study conducted at Weber State University found this particular Magnesium Glycinate was absorbed up to four times more effectively than typical magnesium supplements. Magnesium-the Versatile Mineral The average adult body contains anywhere from about 21 to 28 grams of magnesium. Approximately 60 percent of the body’s magnesium supply is stored in bone. Soft tissue, such as skeletal muscle, contains 38%, leaving only about 1 to 2% of the total body magnesium content in blood plasma and red blood cells. Magnesium in the body may be bound either to proteins or "anions" (negatively charged substances.) About 55% of the body’s magnesium content is in the "ionic" form, which means it carries an electrical charge. Magnesium ions are "cations," ions that carry a positive charge. In its charged state, magnesium functions as one of the mineral "electrolytes." Magnesium works as a "co-factor" for over 300 enzymatic reactions in the body. Metabolism uses a phosphate containing molecule called "ATP" as its energy source. Magnesium is required for all reactions involving ATP [11]. ATP supplies the energy for physical activity, by releasing energy stored in "phosphate bonds". Skeletal and heart muscle use up large amounts of ATP. The energy for muscle contraction is released when one of ATP’s phosphate bonds is broken, in a reaction that produces ADP. Phosphate is added back to ADP, re-forming ATP. ATP also powers the cellular "calcium pump" which allows muscle cells to relax. Because it participates in these ATP-controlled processes, magnesium is vitally important for muscle contraction and relaxation. By controlling the flow of sodium, potassium and calcium in and out of cells, magnesium regulates the function of nerves as well as muscles [12]. Magnesium’s importance for heart health is widely recognized. The heart is the only muscle in the body that generates its own electrical impulses. Through its influence on the heart’s electrical conduction system, magnesium is essential for maintenance of a smooth, regular heartbeat [13]. Magnesium appears to help the heart resist the effects of systemic stress. Magnesium deficiency aggravates cardiac damage due to acute systemic stress (such as caused by infection or trauma), while magnesium supplementation protects the heart against stress [14]. This has been found true even in the absence of an actual magnesium deficit in the body. Evidence suggests that magnesium may help support mineral bone density in elderly women. In a two-year open, controlled trial, 22 out of a group of 31 postmenopausal women who took daily magnesium supplements showed gains in bone density. A control group of 23 women who declined taking the supplements had decreases in bone density [15]. The dietary intakes of magnesium, potassium, fruit and vegetables are associated with increased bone density in elderly women and men [16]. In an interesting animal study, rats were fed diets with either high or low levels of magnesium. Compared to the high magnesium-fed rats, bone strength and magnesium content of bone decreased in the low-magnesium rats, even though these rats showed no visible signs of magnesium deficiency [17]. While this finding may or may not apply to humans, it raises the possibility that diets supplying low magnesium intakes may contribute to weakening of bone in the elderly. Maximizing Absorption––Chelated Minerals Explained Mineral absorption occurs mainly in the small intestine. Like any mineral, magnesium may be absorbed as an "ion," a mineral in its elemental state that carries an electric charge. Mineral ions cross the intestinal membrane either through "active transport" by a protein carrier imbedded in the cells lining the membrane inner wall, or by simple diffusion. The magnesium in mineral salts is absorbed in ionic form. However, absorption of ionic minerals can be compromised by any number of factors, including: 1) Low solubility of the starting salt, which inhibits release of the mineral ion, and 2) Binding of the released ion to naturally occurring dietary factors such as phytates, fats and other minerals that form indigestible mineral complexes [18]. A second absorption mechanism has been discovered for minerals. Experiments have shown that minerals chemically bonded to amino acids (building blocks of protein) are absorbed differently from mineral ions. This has given rise to the introduction of "chelated" minerals as dietary supplements. Mineral amino acid chelates consist of a single atom of elemental mineral that is surrounded by two or more amino acid molecules in a stable, ring-like structure. Unlike mineral salts, which must be digested by stomach acid before the desired mineral portion can be released and absorbed, mineral chelates are not broken down in the stomach or intestines. Instead, chelates cross the intestinal wall intact, carrying the mineral tightly bound and hidden within the amino acid ring. The mineral is then released into the bloodstream for use by the body. Research by pioneers in the field of mineral chelation and human nutrition indicates that the best-absorbed chelates consist of one mineral atom chelated with two amino acids. This form of chelate is called a "di-peptide." Compared to other chelates, di-peptides have the ideal chemical attributes for optimum absorption [19]. Dipeptide chelates demonstrate superior absorption compared to mineral salts. For example, a magnesium di-peptide chelate was shown to be four times better absorbed than magnesium oxide [20]. Consumer Alert! Not all "amino acid chelates" are true chelates. In order for a mineral supplement to qualify as a genuine chelate, it must be carefully processed to ensure the mineral is chemically bonded to the amino acids in a stable molecule with the right characteristics. The magnesium bis-glycinate/lysinate in High Absorption Magnesium is a genuine di-peptide chelate ("bis" means "two"). It has a molecular weight of 324 daltons, considerably lower than the upper limit of 800 daltons stated in the definition of "mineral amino acid chelates" adopted by the National Nutritional Foods Association in 1996 [21]. Bioperine® For Enhanced Absorption Bioperine® is a natural extract derived from black pepper that increases nutrient absorption.* Preliminary trials on humans have shown significant increases in the absorption of nutrients consumed along with Bioperine® [22]. Scientific References 1. Abbott, L.R., R., Clinical manifestations of magnesium deficiency. Miner electrolyte Metab, 1993. 19: p. 314-22. 2. Durlach, J., Recommended dietary amounts of magnesium: Mg RDA. Magnesium Research, 1989. 2(3): p. 195-202. 3. Morgan, K.e.a., Magnesium and calcium dietary intakes of the U.S. population. Journal of the American College of Nutrition, 1985. 4: p. 195-206. 4. Windham, C., Wyse, B., Hurst, R. Hansen, R., Consistency of nutrient consumption patterns in the United States. J AM Diet Assoc, 1981. 78(6): p. 587-95. 5. Pennington, J., Mineral content of foods and total diets: the Selected Minerals in Food Survey, 1982 to 1984. J AM Diet Assoc, 1986. 86(7): p. 876-91. 6. Marier, J., Magnesium Content of the Food Supply in the Modern- Day World. Magnesium, 1986. 5: p. 1-8. 7. Costello, R., Moser-Veillon, P., A review of magnesium intake in the elderly. A cause for concern? Magnesium Research, 1992. 5(1): p. 61-67. 8. Durlach, J., et al., Magnesium status and aging: An update. Magnesium Research, 1997. 11(1): p. 25-42. 9. Seelig, M., Increased need for magnesium with the use of combined oestrogen and calcium for osteoporosis treatment. Magnesium Research, 1990. 3(3): p. 197-215. 10. Zive, M., et al., Marginal vitamin and mineral intakes of young adults: the Bogalusa Heart Study. J Adolesc, 1996. 19(1): p. 39-47. 11. McLean, R., Magnesium and its therapeutic uses: A review. American Journal of Medicine, 1994. 96: p. 63-76. 12. Graber, T., Role of magnesium in health and disease. Comprehensive Therapy, 1987. 13(1): p. 29-35. 13. Sueta, C., Patterson, J., Adams, K., Antiarrhythmic action of pharmacological administration of magnesium in heart failure: A critical review of new data. Magnesium Research, 1995. 8(4): p. 389- 401. 14. Classen, H.-G., Systemic stress, magnesium status and cardiovascular damage. Magnesium, 1986. 5: p. 105-110. 15. Stendig-Lindberg, G., Tepper, R., Leichter, I., Trabecular bone density in a two year controlled trial of peroral magnesium in osteoporosis. Magnesium Research, 1993. 6(2): p. 155-63. 16. Tucker, K., et al., Potassium, magnesium, and fruit and vegetable intakes are associated with greater bone mineral density in elderly men and women. Am J Clin Nutr, 1999. 69(4): p. 727-736. 17. Heroux, O., Peter, D., Tanner, A., Effect of a chronic suboptimal intake of magnesium on magnesium and calcium content of bone and bone strength of the rat. Can J. Physiol. Pharmacol., 1975. 53: p. 304-310. 18. Pineda, O., Ashmead, H.D., Effectiveness of treatment of irondeficiency anemia in infants and young children with ferrous bisglycinate chelate. Nutrition, 2001. 17: p. 381-84. 19. Adibi, A., Intestinal transport of dipetides in man: Relative importance of hydrolysis and intact absorption. J Clin Invest, 1971. 50: p. 2266-75. 20. Ashmead, H.D., Graff, D., Ashmead, H., Intestinal Absorption of Metal Ions and Chelates. 1985, Springfield, Illinois: Charles C. Thomas. 21. NNFA definition of mineral amino acid chlelates, in NNFA Today. 1996. p. 15. 22. Bioperine-Nature's Bioavailability Enhancing Thermonutrient. 1996, Sabinsa Corporation: Piscataway, N.J. *This statement has not been evaluated by the Food and Drug Administration. This product is not intended to diagnose, treat, cure or prevent any disease. Doctor's Best•1120 Calle Cordillera•Suite 101, San Clemente, CA 92673
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=821) Gentle Giant Glycinate - Calcium / Magnesium Glycinate 1:1 ratio 
Date:
July 11, 2005 01:06 PM
Gental Giant Glycinateas you know, minerals come in many forms. Glycinate is the body-friendly gental giant you've been searching for. Calcium and Magnesium Glycinate are fully reacted chelates of calcium and magnesium with the amino acid glycine. Cal Mag Glycinate 1:1 provides 500mg of each mineral in an ActiSorb Base of enhanced absorption. Cal Mag Glycinate 1:1 Your Body will thank you, Actisorb ® Base: (Bioperine [black pepper extract], Ginger root extract, Rosemary Leaf extract, Turmeric root extract, cayenne extract)
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=567) | ||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||